Contents lists available at ScienceDirect journal homepage: www.elsevier.com/locate/envpol
J. Esperschuetz a, N. Balaine a, T. Clough a, S. Bulman b, N.M. Dickinson c, J. Horswell d, B.H. Robinson a, *
a Lincoln University, Faculty of Agriculture and Life Sciences, Department of Soil and Physical Sciences, P O Box 84, Lincoln 7647, New Zealand b Plant and Food Research, Microbiology Division, Canterbury Agriculture and Science Centre, Gerald St, Lincoln 7608, New Zealand c Lincoln University, Faculty of Agriculture and Life Sciences, Department of Ecology, P O Box 84, Lincoln 7647, New Zealand d The Institute of Environmental Science and Research Limited, Kenepuru Science Centre, PO Box 50-348, Porirua 5240, New Zealand
a Lincoln University,农业与生命科学学院,土壤与物理科学系,P O Box 84,Lincoln 7647,新西兰 b Plant and Food Research,微生物学部,Canterbury Agriculture and Science Centre,Gerald St,Lincoln 7608,新西兰 c Lincoln University,农业与生命科学学院,生态学系,P O Box 84,Lincoln 7647,新西兰 d The Institute of Environmental Science and Research Limited,Kenepuru Science Centre,PO Box 50-348,Porirua 5240,新西兰
1Introduction引言
Silvopastoral systems combine forestry and animal production, with trees grown in combination with forage plants and livestock, in an attempt to produce economic returns while minimizing negative impacts on the environment (Lopez-Díaz� et al., 2009). Revenue can be generated from plant products, such as timber (lumber) essential oils and honey, as well as livestock products. Silvopastoral systems may contribute towards sustainable agriculture, and can enhance biodiversity, nutrient cycling efficiency, animal welfare and income (Mosquera-Losada et al., 2005). However, interactions among trees, pasture and animals may pose management difficulties (Eichhorn et al., 2006).
林牧复合系统将林业与畜牧生产相结合,使树木与饲草植物及家畜共同经营,旨在获得经济收益的同时尽量减少对环境的负面影响(Lopez-Díaz et al., 2009)。收入既可来自植物产品,如木材、精油和蜂蜜,也可来自畜产品。林牧复合系统有助于农业的可持续发展,并可提高生物多样性、养分循环效率、动物福利和经济收入(Mosquera-Losada et al., 2005)。然而,树木、牧草与动物之间的相互作用可能给管理带来困难(Eichhorn et al., 2006)。
Trees may compete with pasture for water, nutrients, and above all, light. Therefore species selection and fertilization strategies are critical in optimizing silvopastoral systems (Lopez-Díaz� et al., 2009). After successful plant establishment, fertilization is required to maintain productivity. Urea is the most used N fertilizer in many regions. Following hydrolysis, the ammonium released from urea rapidly nitrifies to nitrate, which can in turn leach or be denitrified and released as nitrogen or nitrous oxide, a potent greenhouse gas (Robertson and Groffman, 2015). Investigations of soil mineral N dynamics show NO3-N concentrations in grazed pastures are 5e10 times higher than NH4-N, indicating these systems are a high nitrifying environment with a high potential for NO3� leaching (Chang et al., 2002; Poudel et al., 2002). In grazed pastures animal urine adds N to the soil at rates of up to 1000 kg N ha�1 (Selbie et al., 2015). This N is far in excess of what can be taken up by pasture and consequently, urine patches are responsible for up to 70% of NO3� leaching in grazed pastures (Cuttle and Bourne, 1993). Trees can reduce NO3� leaching due to their greater effective root depth compared to pasture, which in turn can potentially increase fertilization use efficiency in silvopastoral systems (Mosquera-Losada et al., 2006). Moreover, animals may spend longer under trees that provide shade and shelter (Mosquera- Losada et al., 2005), thereby depositing a disproportionate amount of urine onto the trees’ root zones.
树木可能与牧草竞争水分、养分,尤其是光照。因此,树种选择和施肥策略对于优化林牧复合系统至关重要(Lopez-Díaz et al., 2009)。植物成功定植后,需要施肥以维持生产力。尿素是许多地区使用最多的氮肥。尿素水解释放的铵迅速硝化为硝酸盐,后者可随水淋溶,或经反硝化作用以氮气或氧化亚氮(一种强效温室气体)的形式释放(Robertson and Groffman, 2015)。对土壤矿质氮动态的研究表明,放牧草地中NO3-N浓度是NH4-N的5–10倍,说明这类系统是硝化作用强烈的环境,NO3−淋溶潜力很高(Chang et al., 2002; Poudel et al., 2002)。在放牧草地中,动物尿液向土壤输入的氮可高达1000 kg N ha−1(Selbie et al., 2015)。这一氮量远超牧草所能吸收的量,因此尿斑导致的NO3−淋溶可占放牧草地该类淋溶总量的70%(Cuttle and Bourne, 1993)。与牧草相比,树木的有效根深更大,可减少NO3−淋溶,进而有望提高林牧复合系统的肥料利用效率(Mosquera-Losada et al., 2006)。此外,动物可能在提供遮荫和庇护的树下停留更长时间(Mosquera- Losada et al., 2005),从而在树木根区排泄不成比例的大量尿液。
* This paper has been recommended for acceptance by Klaus Kummerer.
* 本文经Klaus Kummerer推荐录用。
* Corresponding author. E-mail address: brett.robinson@lincoln.ac.nz (B.H. Robinson).
Nitrification rates may be affected by both trees and herbaceous species. Plants may enhance or inhibit nitrification, via root exudates (Subbarao et al., 2009) or compounds released into the soil from abscised leaves (Northup et al., 1995; Paavolainen et al., 1998). Such biological nitrification inhibition (BNI) occurs due to the inhibition of enzymes that are involved in the nitrification process (Subbarao et al., 2013), or by changing microbial communities in soil (Amaral et al., 1998). Nitrification inhibiting properties have been reported for polyphenolic compounds (Castaldi et al., 2009; Rice and Pancholy, 1973) or monoterpenes (White, 1988), which are commonly found in pine litter (Northup et al., 1995). P. radiata stands have been observed to inhibit nitrification in a New Zealand field site (Cooper, 1986), and leaf extracts decreased nitrification in soil incubation trials (Suescun et al., 2012). Inhibiting nitrification subsequently affects denitrification, since less NO3� is available as substrate for N2O production. Plant species with BNI properties can potentially reduce N2O losses associated with nitrification (Subbarao et al., 2013). Monterey pine (Pinus radiata D. Don) is one of the world's commercially dominant tree species, and is well integrated in silvopastoral systems in temperate areas such as Australia, New Zealand and Chile (Lopez-Díaz� et al., 2009). However, decreases in log prices have reduced the incentive to replant harvested trees. In New Zealand and elsewhere, there is increasing interest in incorporating native species into farming systems to improve the quality of surface waters (Franklin et al., 2015). Manuka (� Leptospermum scoparium J.R. Forst & G. Forst) and kanuka� (Kunzea robusta de Lange & Toelken) are in the myrtaceae family and are common throughout New Zealand and Australia (Bergin et al., 1995; Stephens et al., 2005). Both, m�anuka and kanuka� are attracting interest due to their role in the production of essential oils (Maddocks-Jennings et al., 2005; Song et al., 2013) and honey (Beitlich et al., 2014; Steinhorn et al., 2011). Compounds associated with manuka� and k�anuka have demonstrable antimicrobial properties (Prosser, 2011; Wyatt et al., 2005). Prosser et al. (2016) found that manuka� killed E. coli in soil. We hypothesise that these antimicrobial compounds associated with these species may affect N cycling, which is microbially mediated and therefore reduce N leaching or gaseous N emissions (Castaldi et al., 2009; White,1988).
硝化速率可能同时受到树木和草本植物的影响。植物可通过根系分泌物(Subbarao et al., 2009)或凋落叶释放到土壤中的化合物(Northup et al., 1995; Paavolainen et al., 1998)促进或抑制硝化作用。这种生物硝化抑制(BNI)源于对参与硝化过程的酶的抑制(Subbarao et al., 2013),或源于土壤微生物群落的改变(Amaral et al., 1998)。已有报道表明,多酚类化合物(Castaldi et al., 2009; Rice and Pancholy, 1973)或单萜类化合物(White, 1988)具有硝化抑制特性,而这些物质常见于松树凋落物中(Northup et al., 1995)。在新西兰的一处田间样地中观察到P. radiata林分可抑制硝化作用(Cooper, 1986),在土壤培养试验中其叶片提取物也降低了硝化作用(Suescun et al., 2012)。抑制硝化作用进而会影响反硝化作用,因为可作为N2O生成底物的NO3−减少。具有BNI特性的植物物种有望减少与硝化作用相关的N2O损失(Subbarao et al., 2013)。辐射松(Pinus radiata D. Don)是世界上商业上占主导地位的树种之一,已广泛纳入澳大利亚、新西兰和智利等温带地区的林牧复合系统(Lopez-Díaz et al., 2009)。然而,原木价格下跌降低了采伐后重新造林的积极性。在新西兰及其他地区,人们越来越关注将本土物种纳入农业系统以改善地表水质量(Franklin et al., 2015)。麦卢卡(Leptospermum scoparium J.R. Forst & G. Forst)和卡努卡(Kunzea robusta de Lange & Toelken)同属桃金娘科,广泛分布于新西兰和澳大利亚(Bergin et al., 1995; Stephens et al., 2005)。麦卢卡和卡努卡因其在精油(Maddocks-Jennings et al., 2005; Song et al., 2013)和蜂蜜(Beitlich et al., 2014; Steinhorn et al., 2011)生产中的作用而受到关注。与麦卢卡和卡努卡相关的化合物具有明确的抗菌特性(Prosser, 2011; Wyatt et al., 2005)。Prosser et al.(2016)发现麦卢卡可杀灭土壤中的E. coli。我们假设,这些物种相关的抗菌化合物可能影响由微生物介导的氮循环,从而减少氮淋溶或气态氮排放(Castaldi et al., 2009; White,1988)。
Manuka� and k�anuka are adapted to low fertility environments, hence their growth responses to N resulting from fertilization or animal excreta in agricultural systems are unknown (Franklin et al., 2015), whereas pine responds positively to N (Neilsen et al., 1992). Increasing biomass production by fertilization while simultaneously minimizing N losses from these systems could enhance the sustainability of silvopastoral systems, while increasing productivity and revenue due to the high-grade timber and plant related products, such as honey and essential oils (Porter and Wilkins, 1999; Stephens et al., 2010).
麦卢卡和卡努卡适应低肥力环境,因此其对农业系统中施肥或动物排泄物所带来的氮的生长响应尚不清楚(Franklin et al., 2015),而松树对氮呈正响应(Neilsen et al., 1992)。通过施肥提高生物量产量,同时尽量减少这些系统的氮损失,可增强林牧复合系统的可持续性,并借助优质木材及蜂蜜、精油等植物相关产品提高生产力和收益(Porter and Wilkins, 1999; Stephens et al., 2010)。
We aimed to determine whether urea could increase the biomass production of manuka� and kanuka� and the potential of these species to reduce N2O-emissions and NO3� leaching in silvopastoral systems. We sought to compare these with Pinus radiata, which is common in silvopastoral systems, responds positively to N, and has allochemicals that inhibit nitrification.
本研究旨在确定尿素能否提高麦卢卡和卡努卡的生物量产量,以及这些物种在林牧复合系统中减少N2O排放和NO3−淋溶的潜力。我们将其与Pinus radiata进行比较,后者在林牧复合系统中较为常见,对氮呈正响应,且含有抑制硝化作用的化感物质。
a marginal slope of the North Island New Zealand near Bideford (40�4505600S 175�5404200E), which was representative of many low fertility soils under native vegetation, dominated by m�anuka (L. scoparium) and kanuka (� K. robusta). Soil analyses showed the soil was pH 6.1, with a medium carbon (6.5%) and N (0.46%) level, a C/N ratio of 14.3 and a low level of bicarbonate (Olsen) extractable phosphorus (11 mg L�1). Cation exchange capacity (CEC) was determined at 21 me 100 g�1. To measure NO3� leaching, a leachatesampling device was installed in the bottom of each lysimeter, covered by fleece sheets and a gravel drainage layer to avoid stagnant moisture.
新西兰北岛Bideford附近的一处边际坡地(40°45′56″S 175°54′42″E),该土壤代表了本土植被下的许多低肥力土壤,植被以麦卢卡(L. scoparium)和卡努卡(K. robusta)为主。土壤分析表明,该土壤pH为6.1,碳(6.5%)和氮(0.46%)含量中等,C/N比为14.3,碳酸氢盐(Olsen)可提取磷含量较低(11 mg L−1)。阳离子交换量(CEC)测定值为21 me 100 g−1。为测定NO3−淋溶,在每个渗漏计底部安装了渗滤液采样装置,其上覆盖无纺布和砾石排水层,以避免积水。
Two native New Zealand trees, manuka� and k�anuka, as well as pine, were grown with or without urea fertilizer, replicated four times. All species were planted into the lysimeters on the 6th of August 2013, after they had been filled and settled for eight weeks. P. radiata seedlings (GF19) were purchased from Southern Woods Nursery Ltd, Christchurch/New Zealand. L. scoparium (PH lebsco, 6M) and K. robusta (KV kunert, 6M) were purchased from Wai-ora Nursery Ltd, Christchurch/New Zealand. All seedlings were purchased in rootrainers at a seedling size of between 35 and 50 cm. To allow N2O measurements, a chamber base for gas sampling (10 cm in diameter and 10 cm in height) was installed (5 cm deep) into each lysimeter. After all plants have been established in the lysimeters for six weeks, urea was applied onto the lysimeters. The urea treatments received an equivalent of 200 kg N ha�1 in total, which is the maximum allowable annual rate that N can be applied in most NZ jurisdictions (Pyke et al., 2016). The urea application occurred as four 0.53 g applications per lysimeter, equivalent to 50 kg ha�1 each application on September 16th, October 7th, October 29th and November 18th of 2013. Control treatments did not receive any urea.
两种新西兰本土树种麦卢卡和卡努卡以及松树分别在施用或不施用尿素的条件下种植,每个处理重复4次。渗漏计装土并沉降8周后,于2013年8月6日将所有物种栽入渗漏计。P. radiata幼苗(GF19)购自新西兰基督城Southern Woods Nursery Ltd。L. scoparium(PH lebsco,6M)和K. robusta(KV kunert,6M)购自新西兰基督城Wai-ora Nursery Ltd。所有幼苗均为育苗容器苗,苗高35–50 cm。为进行N2O测定,在每个渗漏计中安装了用于气体采样的箱体底座(直径10 cm,高10 cm,埋深5 cm)。所有植株在渗漏计中定植6周后施用尿素。尿素处理共施加相当于200 kg N ha−1的氮,这是新西兰大多数行政辖区允许的最高年施氮量(Pyke et al., 2016)。尿素分4次施用,每个渗漏计每次0.53 g,相当于每次50 kg ha−1,施用日期分别为2013年9月16日、10月7日、10月29日和11月18日。对照处理不施尿素。
Prior to final harvest, a urea application of 8.48 g of urea (800 kg N ha�1 equiv.) was carried out, simulating a ruminant urine event commonly occurring in farm systems (Oenema et al., 1997; Selbie et al., 2015). This high N application was followed by N2O measurements for 20 days. For N2O measurement, a polypropylene chamber was placed over the permanently installed ring for 40 min and sealed with a worm drive hose clip, resulting in a headspace volume of 500 mL. Samples were taken immediately after chamber placement (t0), after 20 (t1) as well as 40 min (t2) with a syringe and needle inserted at a rubber septum on top of the chamber. The greenhouse temperature during the time of N2O measurement was recorded for flux calculations (Fig. S1 - Supplemental material).
最终收获前,施用8.48 g尿素(相当于800 kg N ha−1),以模拟农业系统中常见的反刍动物排尿事件(Oenema et al., 1997; Selbie et al., 2015)。高量施氮后连续20天测定N2O。测定N2O时,将聚丙烯箱罩于永久安装的底座环上40 min,并用蜗杆式软管卡箍密封,顶空体积为500 mL。分别在罩箱后立即(t0)、20 min(t1)和40 min(t2)时,用注射器和针头经箱顶橡胶隔垫采集气样。记录N2O测定期间的温室温度,用于通量计算(图S1 - 补充材料)。
Watering during the experimental period was carried out via an automated irrigation system, which allowed an independent watering of each plant species by pressure compensated drippers. Irrigation was controlled and adjusted daily to provide at ca. of 20e30 mm of drainage per week to account for differing rates of evapotranspiration and near-field capacity conditions.
试验期间采用自动灌溉系统浇水,通过压力补偿滴头对每种植物进行独立灌溉。每日控制和调整灌溉量,使每周排水量约为20–30 mm,以兼顾不同的蒸散速率并维持接近田间持水量的条件。
A final destructive harvest of all lysimeters was performed after 20 days of N2O measurement. The above-ground and belowground plant biomass were weighed and oven-dried at 60 �C until a constant weight, carefully separated and reweighed. Soil attached to the roots �2 mm was considered as rhizosphere soil. Rhizosphere soil was harvested, subsampled and stored for further analyses at 4 �C after sieving �5 mm.
N2O测定20天后,对所有渗漏计进行最终破坏性收获。地上和地下植物生物量称重后,在60 °C下烘干至恒重,仔细分离后再次称重。附着在根系上的≤2 mm土壤视为根际土壤。收获根际土壤,过≤5 mm筛后分取子样,于4 °C下保存以供进一步分析。
2.1. Analyses and measurements2.1. 分析与测定
2Material and methods材料与方法
In May 2013, 10 L lysimeters were constructed and installed at the Lincoln University plant growth facility (43�3804200S 172�2704100E). Each lysimeter was filled with 10 L of soil at an average soil bulk density of 1.0 g cm�33. The soil was collected from
2013年5月,在Lincoln University植物生长设施(43°38′42″S 172°27′41″E)建造并安装了10 L渗漏计。每个渗漏计装入10 L土壤,平均土壤容重为1.0 g cm−3。土壤采自
Soil pH was measured from rhizosphere soil samples by adding 25 mL of DI water to 15 g of fresh soil (Blakemore et al., 1987). Total N in plant and soil material was analysed using oven dried (60 �C) and ground material using a CNS-2000 Element Analyser (LECO Australia Pty Ltd, Australia). In order to investigate the influence of the plant species on N transformation and translocation into the soil, the rhizosphere soil was used to determine the soil inorganic N speciation. A KCl extraction was carried out from fresh soil (4 �C) within 4 days after harvest according to (Blakemore et al., 1987). After adding 40 mL of a 2M KCl reagent to 4 g of soil, the solution was shaken on an end-over-end shaker for 1 h, centrifuged at 827 g for 10 min and subsequently filtered through Whatman 41 filter paper. Nitrate-N (NO3-N) and ammonium-N (NH4-N) were determined using a flow injection analyser (FIA FS3000 twin channel analyser, Alpkem, USA). Leachate samples were kept at �20 �C until FIA analyses.
根际土壤样品的pH测定方法为向15 g新鲜土壤中加入25 mL去离子水(Blakemore et al., 1987)。植物和土壤样品的全氮采用烘干(60 °C)并磨碎的样品,用CNS-2000元素分析仪(LECO Australia Pty Ltd,澳大利亚)测定。为研究植物物种对氮转化及其向土壤迁移的影响,采用根际土壤测定土壤无机氮形态。收获后4天内,按照(Blakemore et al., 1987)的方法对新鲜土壤(4 °C)进行KCl提取。向4 g土壤中加入40 mL 2M KCl试剂后,在翻转振荡器上振荡1 h,以827 g离心10 min,随后用Whatman 41滤纸过滤。硝态氮(NO3-N)和铵态氮(NH4-N)采用流动注射分析仪(FIA FS3000双通道分析仪,Alpkem,美国)测定。渗滤液样品在−20 °C下保存直至进行FIA分析。
Samples for N2O flux calculations were taken for both, control and urea treatments. Nitrous oxide concentration was determined using a gas chromatograph (GC) (SRI 8610 gas chromatograph; SRI Instruments, CA, USA) equipped with a63Ni electron capture detector (ECD) and autosampler (Gilson 222 XL; Gilson Inc., WI, USA). The GC was calibrated using a series of standard gases interspersed with reference standards. The N2O flux was calculated from the concentration obtained via GC analysis (mL L�1), by integrating the calculated daily N2O fluxes and linearly interpolating between measurement points for each lysimeter after equation (1) according to (Hutchinson and Mosier, 1981), where Vc represents the chamber volume of 0.0005 m3, P the atmospheric pressure of 101325 Pa, c0 and c2 the N2O concentration [mL L�1] at time t0 and t2, respectively, C the amount of minutes per hour (60), M the molecular weight of N2O-N (28.0134 g mol�1), Gc the gas constant (8.314 J K�1 mol�1), Tk the absolute temperature at 0� (273.15 K), Tc the air temperature during measurement (�C), Ac the chamber area (0.0057 m2) and t2 the total cover period of 40 min. The total N2O flux (mg N2O-N m�2 h�1) was converted and illustrated as cumulative daily flux per hectare for illustrations and comparison with other N parameters.
对照和尿素处理均采集了用于计算N2O通量的样品。氧化亚氮浓度采用配备63Ni电子捕获检测器(ECD)和自动进样器(Gilson 222 XL;Gilson Inc.,WI,美国)的气相色谱仪(GC)(SRI 8610气相色谱仪;SRI Instruments,CA,美国)测定。GC采用一系列标准气体并穿插参比标准进行校准。N2O通量由GC分析所得浓度(mL L−1)计算,按照(Hutchinson and Mosier, 1981)的式(1)对每个渗漏计计算日N2O通量,并在测定点之间线性插值后积分得到;式中Vc为箱体体积0.0005 m3,P为大气压101325 Pa,c0和c2分别为t0和t2时的N2O浓度[mL L−1],C为每小时的分钟数(60),M为N2O-N的分子量(28.0134 g mol−1),Gc为气体常数(8.314 J K−1 mol−1),Tk为0°时的绝对温度(273.15 K),Tc为测定期间的气温(°C),Ac为箱体面积(0.0057 m2),t2为总罩箱时间40 min。总N2O通量(mg N2O-N m−2 h−1)经换算后以每公顷累积日通量表示,用于作图及与其他氮参数的比较。
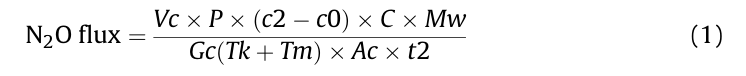
A soil nitrification assay performed using the rhizosphere control soil and an (NH4)2SO4 solution (10 g of fresh soil in 100 mL working solution). The (NH4)2SO4 solution was set up with 1.5 mL of 0.2 M KH2PO4 and 15 mL of 50 mM (NH4)2SO4�, which was diluted to 1 L. The pH of the diluted solution was adjusted to 7.2 by addition of H2SO4 and NaOH, respectively. The soil slurry was shaken at 150 rpm and incubated at 28 �C for 4 weeks, with measurements taken for NO3� and NH4+ after filtering on days 0, 1, 3, 7 and 24.
采用对照根际土壤和(NH4)2SO4溶液进行土壤硝化试验(10 g新鲜土壤加入100 mL工作液)。(NH4)2SO4溶液由1.5 mL 0.2 M KH2PO4和15 mL 50 mM (NH4)2SO4−配制,并稀释至1 L。分别加入H2SO4和NaOH将稀释液pH调至7.2。土壤悬浮液以150 rpm振荡,于28 °C下培养4周,并于第0、1、3、7和24天过滤后测定NO3−和NH4+。
Statistical analyses were based on n = 4 individual replicates unless stated otherwise. Using SPSS (IBM SPSS statistics 20), data were tested for normality (Kolmogorov-Smirnov) and if necessary, log-transformed prior analyses of variance (ANOVA) followed by Duncan's post-hoc tests to identify homogenous subsets for a = 0.05. SigmaPlot 11.0 (Systat Software Inc) was used for illustrations.
除另有说明外,统计分析均基于n = 4个独立重复。采用SPSS(IBM SPSS statistics 20)对数据进行正态性检验(Kolmogorov-Smirnov),必要时经对数转换后进行方差分析(ANOVA),随后采用Duncan事后检验确定α = 0.05水平下的同质子集。采用SigmaPlot 11.0(Systat Software Inc)作图。
3Results结果
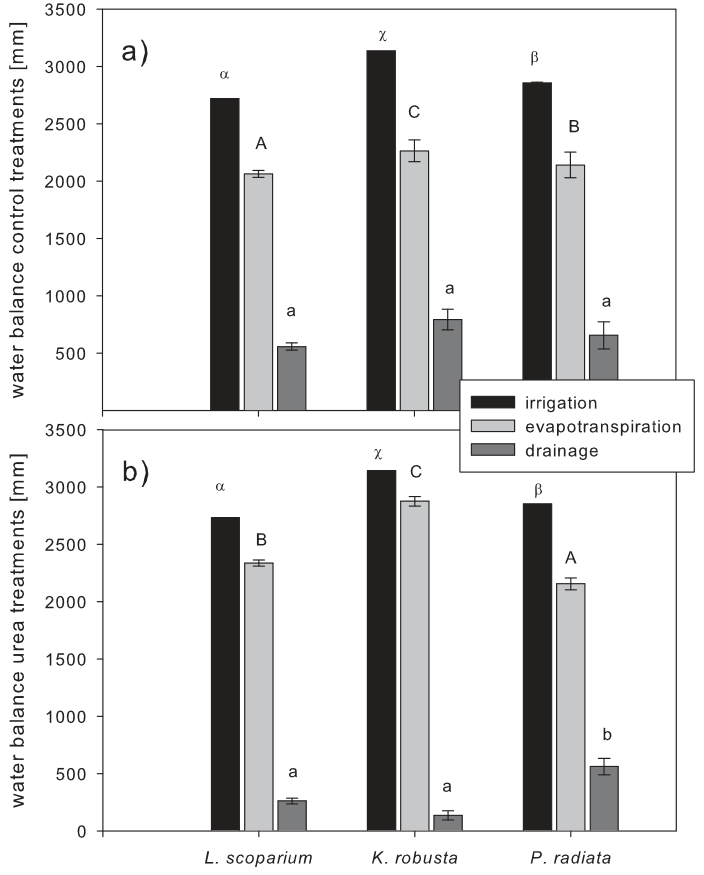
In both the control and the treatments, the total irrigation for m�anuka, kanuka,� and pine was 2730, 3140, and 2850 mm respectively (Fig. 1). Leachate was obtained from all species and treatments over the experimental period, although a slightly higher evapotranspiration in combination with lower drainage was observed in the kanuka and m� �anuka treatments when compared to pine.
在对照和处理中,麦卢卡、卡努卡和松树的总灌溉量分别为2730、3140和2850 mm(图1)。试验期间所有物种和处理均获得了渗滤液,但与松树相比,卡努卡和麦卢卡处理的蒸散量略高,排水量较低。
Soil pH was not significantly different between plant species within treatments, but was significantly lower after urea application in all treatments (Table 1). At final harvest, soil bulk density and water filled pore space were similar in all plant species in control treatments. In urea treatments a lower bulk density was measured in P. radiata compared to L. scoparium, whereas the water filled pore space was higher in P. radiata compared to L. scoparium. The water filled pore space and soil moisture content was detected as significantly lower in urea treatments of both, L. scoparium and K. robusta compared to their corresponding controls. A higher moisture content was measured in P. radiata compared to L. scoparium or K. robusta, irrespective of treatments.
同一处理内不同植物物种间土壤pH无显著差异,但施用尿素后所有处理的土壤pH均显著降低(表1)。最终收获时,对照处理中所有植物物种的土壤容重和充水孔隙度相近。在尿素处理中,P. radiata的土壤容重低于L. scoparium,而充水孔隙度则高于L. scoparium。L. scoparium和K. robusta尿素处理的充水孔隙度和土壤含水量均显著低于其相应对照。无论何种处理,P. radiata的含水量均高于L. scoparium或K. robusta。
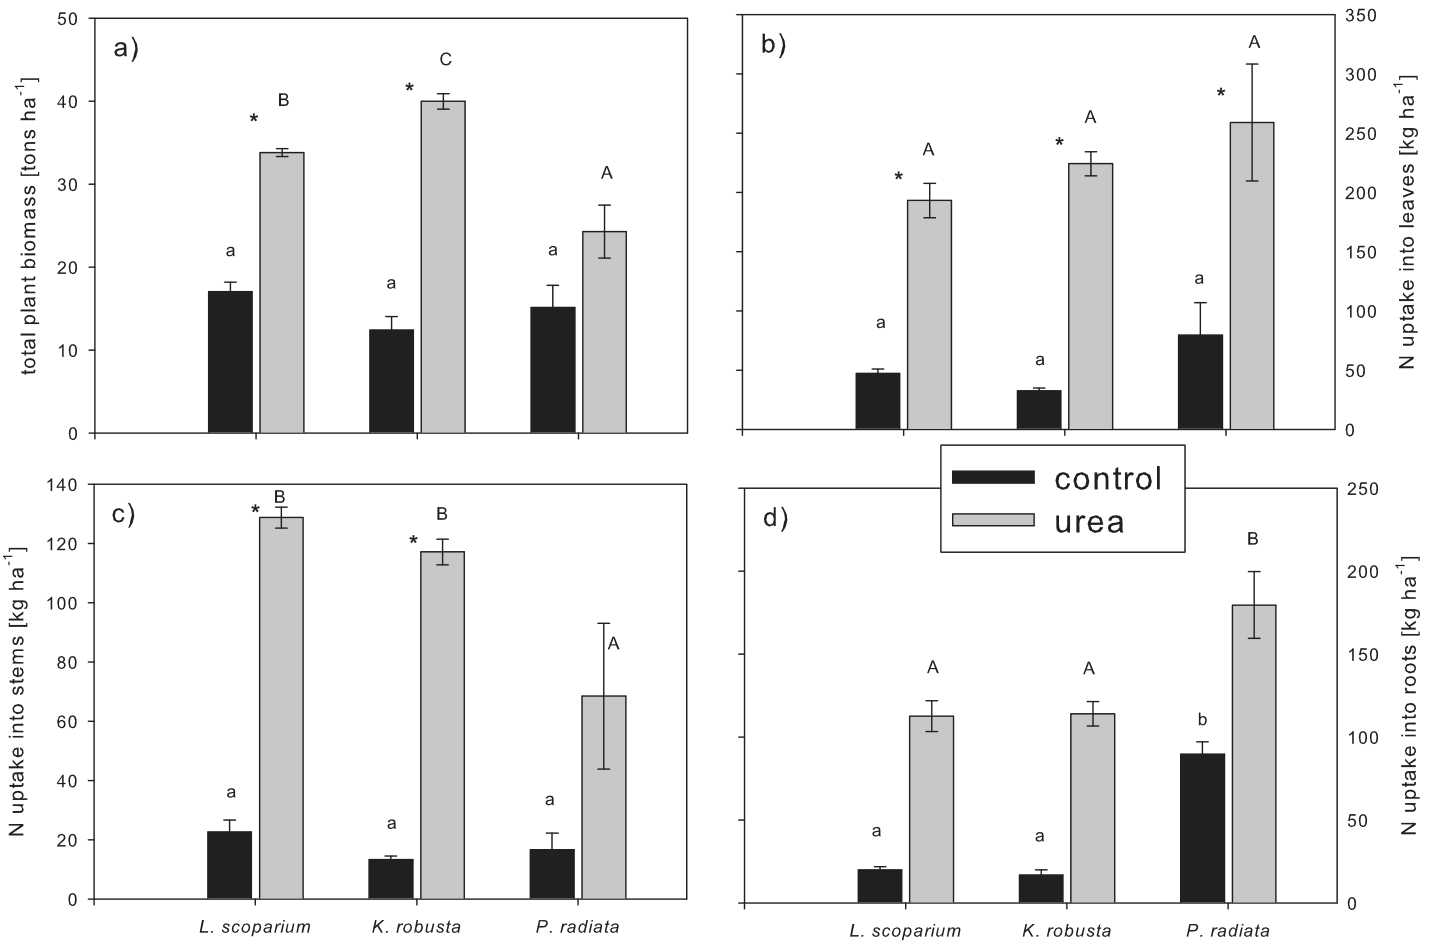
Urea application resulted in significantly increased (p < 0.05) aboveground plant biomass (Fig. 2a) and higher N uptake (p < 0.05) into plant leaves, stems and roots compared to control treatments, irrespective of plant species (Fig. 2b, c, 2d). Pine, manuka� and kanuka� had similar leaf N uptake (Fig. 2b). Lower N content was detected in pine stems (Fig. 2c) compared to both myrtaceae species, whereas higher N content was detected in roots (Fig. 2d).
与对照处理相比,无论何种植物物种,施用尿素均使地上植物生物量显著增加(p < 0.05)(图2a),且叶片、茎和根系的氮吸收量更高(p < 0.05)(图2b、c、2d)。松树、麦卢卡和卡努卡的叶片氮吸收量相近(图2b)。与两种桃金娘科物种相比,松树茎中氮含量较低(图2c),而根系中氮含量较高(图2d)。
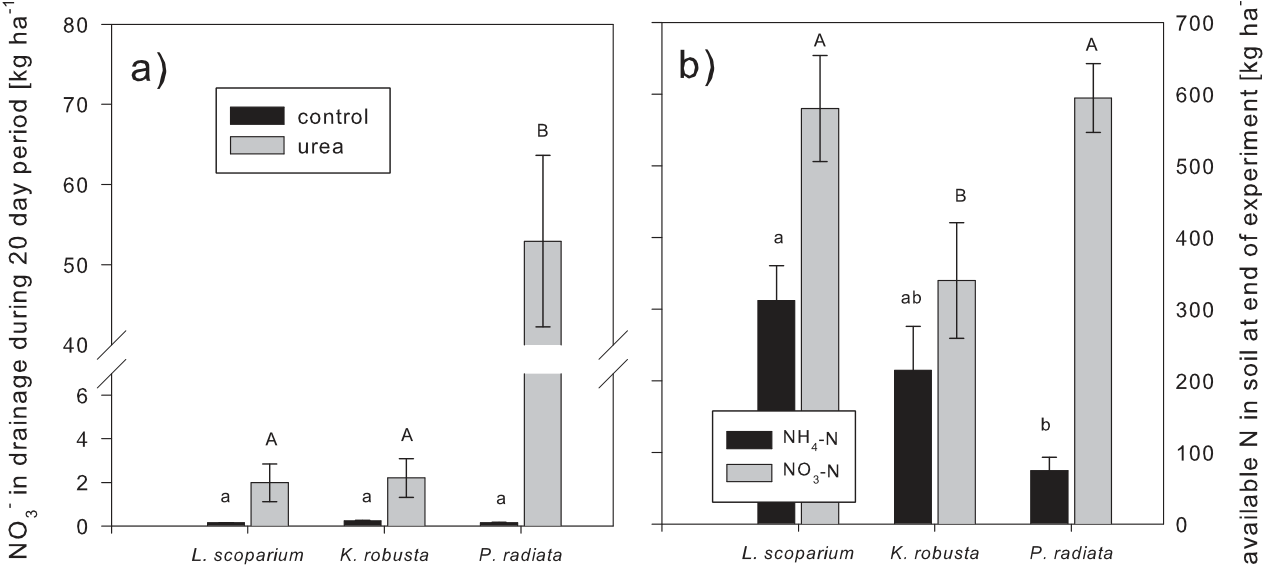
Cumulative NO3�-N leached during the 20-day period was <0.5 kg ha�1 in plant species controls (Fig. 3a). In both myrtaceae species, ca. 2 kg ha�1 NO3�-N were recovered from urea treatments, whereas pine leached 53 kg ha�1 (Fig. 3a). At the end of the experiment, a similar N content (5650e5810 kg ha�1) was measured in the control treatments of all plant species. Urea application increased total N in soil in all plant treatments (6085e6267 kg ha�1). Available N was below the detection limit in control treatments of all plant species (0.1 mg L�1, equivalent to 5 mg kg�1 soil). In urea treatments, NO3�-N was the dominant form of inorganic N in all plant species, although not statistically significant for kanuka� (Fig. 3b). Lower amounts of NO3�-N were detected in urea treatments with kanuka, compared to m� anuka and� pine. Higher levels of NH4+-N were found in both, kanuka� and manuka� compared to pine trees (Fig. 3b).
在20天期间,各植物物种对照处理的累积NO3−-N淋溶量均<0.5 kg ha−1(图3a)。两种桃金娘科物种的尿素处理中回收的NO3−-N约为2 kg ha−1,而松树的淋溶量为53 kg ha−1(图3a)。试验结束时,所有植物物种对照处理的氮含量相近(5650–5810 kg ha−1)。施用尿素使所有植物处理的土壤全氮增加(6085–6267 kg ha−1)。所有植物物种对照处理的有效氮均低于检出限(0.1 mg L−1,相当于5 mg kg−1土壤)。在尿素处理中,NO3−-N是所有植物物种无机氮的主要形态,但卡努卡的差异未达显著水平(图3b)。与麦卢卡和松树相比,卡努卡尿素处理中检测到的NO3−-N较低。与松树相比,卡努卡和麦卢卡中的NH4+-N水平较高(图3b)。
Soil pH, soil bulk density, gravimetric water content and water filled pore space at final harvest [n = 4 ± se]. Significant differences between plant species at p � 0.05 are indicated by letters (a, b, c), considering the same treatment. Differences between treatments within the same plant species are indicated with asterisks (*).
最终收获时的土壤pH、土壤容重、质量含水量和充水孔隙度(n = 4 ± se)。在同一处理下,植物物种间p ≤ 0.05水平的显著差异以字母(a, b, c)表示。同一植物物种不同处理间的差异以星号(*)表示。
| control对照 | urea尿素 | ||
|---|---|---|---|
| soil pH | L.scoparium | 6.28 ± 0.03; 0.03a, * | 5.45 ± 0.06; 0.05a, * |
| K. robusta | 6.33 ± 0.02; 0.02a, * | 5.57 ± 0.03; 0.02a, * | |
| P. radiata | 6.12 ± 0.15; 0.11a, * | 5.38 ± 0.10; 0.08a, * | |
| soil bulk density [g cm�3] | L.scoparium | 0.74 ± 0.04a | 0.80 ± 0.01b |
| K. robusta | 0.81 ± 0.04a | 0.73 ± 0.02ab | |
| P. radiata | 0.75 ± 0.03a | 0.65 ± 0.05a | |
| gravimetric water content [g g�1] | L.scoparium | 33.75 ± 1.18a, * | 16.75 ± 2.10a, * |
| K. robusta | 32.50 ± 1.32a, * | 23.00 ± 2.04b, * | |
| P. radiata | 39.00 ± 0.00b | 41.25 ± 1.11c | |
| water filled pore space [cm3 cm�3] | L.scoparium | 0.34 ± 0.02a, * | 0.19 ± 0.02a, * |
| K. robusta | 0.38 ± 0.03a, * | 0.23 ± 0.03a, * | |
| P. radiata | 0.32 ± 0.11a | 0.36 ± 0.04b |
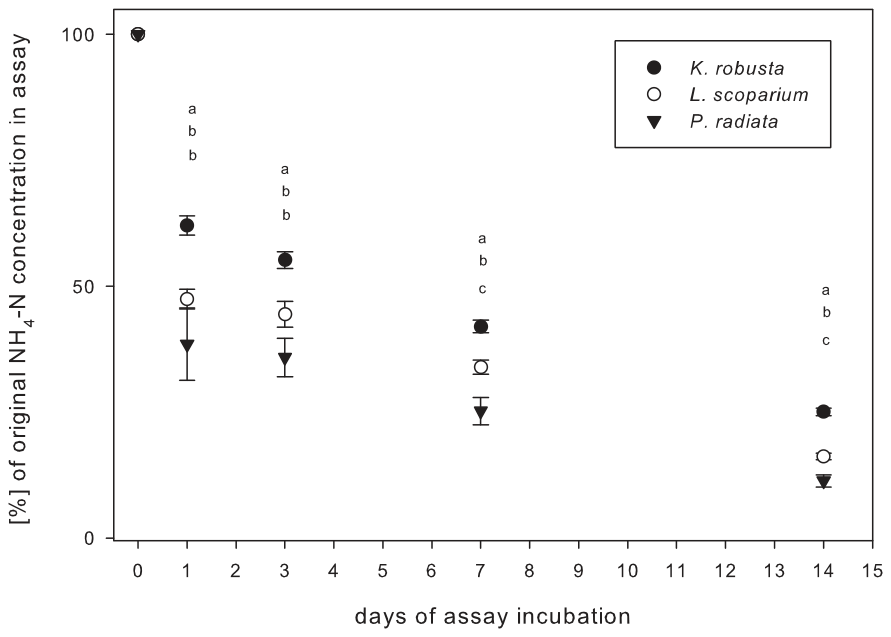
Results from the nitrification assay showed significantly higher concentrations of NH4+-N in kanuka� after only one day of assay incubation, and all subsequent incubation measurements (Fig. 4). After an incubation period of 7 days and 14 days, respectively, higher amounts of NH4+-N were detected in K. robusta compared to L. scoparium, whereas samples from P. radiata being lowest (p < 0.05).
硝化试验结果表明,仅培养1天后卡努卡中的NH4+-N浓度即显著较高,且在随后所有培养测定中均如此(图4)。分别培养7天和14天后,K. robusta中检测到的NH4+-N高于L. scoparium,而P. radiata样品最低(p < 0.05)。
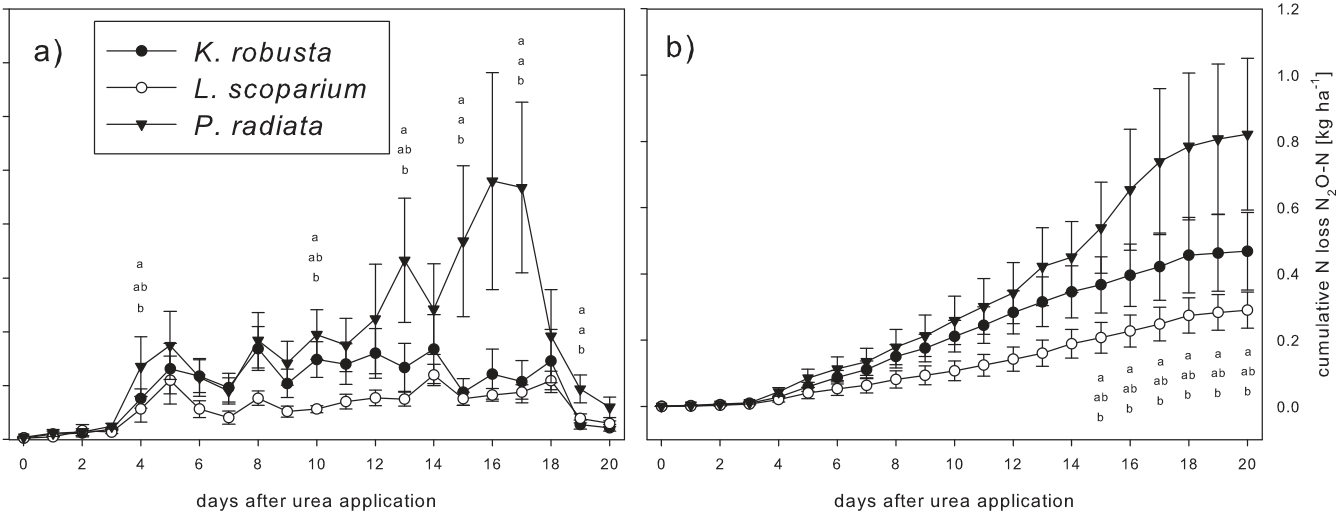
A control N2O-N flux of <10 mg m�2 h�1 was measured in combination with all plant species, resulting in a cumulative N2O-N loss <0.02 kg ha�1 (Fig. S2 e supplemental material). Urea application increased N2O emissions. A moderate increase was measured for all plant species until day 5, where N2O emissions increased up to 110 mg m�2 h�1, 131 mg m�2 h�1 and 174 mg m�2 h�1, in manuka,� kanuka� and pine, respectively (Fig. 5a). In pine treatments, continuously high N2O fluxes were measured until day 17 (468 mg m�2 h�1), followed by decreasing fluxes at the end of the measuring period. In kanuka,� N2O flux was mainly in a range between 120 and 170 mg m�2 h�1, until day 18, and dropped back to 22 mg m�2 h�1 at day 20. The N2O flux measured in urea treatments in combination with manuka was lowest of all plant species, with a� first peak at day 5 (110 mg m�2 h�1) and a second peak at day 14 of the measuring period (120 mg m�2 h�1). The cumulative N loss via N2O over the 20-day period after urea application was 0.82 ± 0.23 kg ha�1, 0.47 ± 0.18 kg ha�1 and 0.29 ± 0.05 kg ha�1, in pine, kanuka� and manuka,� respectively (Fig. 5b).
所有植物物种对照处理的N2O-N通量均<10 mg m−2 h−1,累积N2O-N损失<0.02 kg ha−1(图S2 - 补充材料)。施用尿素增加了N2O排放。至第5天,所有植物物种的N2O排放均呈中等程度增加,麦卢卡、卡努卡和松树的N2O排放分别升至110 mg m−2 h−1、131 mg m−2 h−1和174 mg m−2 h−1(图5a)。松树处理中直至第17天均测得持续较高的N2O通量(468 mg m−2 h−1),此后在测定期末通量下降。卡努卡的N2O通量在第18天前主要介于120和170 mg m−2 h−1之间,至第20天回落至22 mg m−2 h−1。麦卢卡尿素处理测得的N2O通量在所有植物物种中最低,在测定期第5天出现第一个峰值(110 mg m−2 h−1),第14天出现第二个峰值(120 mg m−2 h−1)。施用尿素后20天内经N2O途径的累积氮损失,松树、卡努卡和麦卢卡分别为0.82 ± 0.23 kg ha−1、0.47 ± 0.18 kg ha−1和0.29 ± 0.05 kg ha−1(图5b)。
4Discussion讨论
The trees in the control soils all grew without any visible deficiency symptoms. This demonstrates that they are adapted to low fertility soil and marginal land, and hence have potential use in silvopastoral systems, shelterbelts or marginal farm areas (Hawke and Tombleson, 1993). Manuka� and kanuka� in such systems show potential as nurse crops for underlying vegetation (Herbert et al., 1997). Urea fertilization increased the aboveground biomass of all tree species, especially kanuka and m� �anuka. This was accompanied by an increased evapotranspiration and lower drainage, when compared to pine by similar irrigation pattern (2730 mme3140 mm). The better response of manuka and k� anuka� to urea fertilization compared to pine may indicate that these species could potentially remove more excess N from soil and hence reduce N leaching (Mohan Kumar et al., 1998).
对照土壤中的树木均正常生长,未出现任何可见的缺素症状。这表明它们适应低肥力土壤和边际土地,因而有望用于林牧复合系统、防护林带或农场边际区域(Hawke and Tombleson, 1993)。在此类系统中,麦卢卡和卡努卡具有作为下层植被保育作物的潜力(Herbert et al., 1997)。尿素施肥提高了所有树种的地上生物量,尤其是卡努卡和麦卢卡。在灌溉模式相近(2730–3140 mm)的条件下,与松树相比,这伴随着更高的蒸散量和更低的排水量。与松树相比,麦卢卡和卡努卡对尿素施肥的响应更好,这可能表明这些物种能够从土壤中移除更多过量的氮,从而减少氮淋溶(Mohan Kumar et al., 1998)。
After application of 800 kg ha�1 of urea, similar N was measured in plant leaves, irrespective of plant species. An increased foliar N content was shown to be beneficial for essential oil production in Zingiber officinale (Singh et al., 2016). With increased N fertilization, Tsamaidi et al. (2012) reported an increase in the essential oil yield of dill, containing a-pinene and myrcene, which are key components in manuka,� kanuka� and pine essential oils (McDonald et al., 1999; Porter et al., 1998; Porter and Wilkins, 1999). These tree species included in silvopastoral systems could generate revenue via increased amounts and/or quality of essential oils, obtained through N fertilization or via interruption of stock urine patches. Further studies are needed to determine whether the urea changes the quality of any plant products. In N fertilized treatments both manuka� and kanuka� allocated 100 kg N ha�1 in the stem biomass, compared to only 35 kg ha�1 in pine, whereas N allocation belowground was similar for all tree species (90e100 kg ha�1). These results indicate a better response of manuka� and k�anuka to urea fertilization regarding harvestable aboveground (timber) products.
施用800 kg ha−1尿素后,无论何种植物物种,叶片中测得的氮含量相近。已有研究表明,提高叶片氮含量有利于Zingiber officinale的精油生产(Singh et al., 2016)。Tsamaidi et al.(2012)报道,随着施氮量增加,莳萝的精油产量提高,其精油含有α-蒎烯和月桂烯,而这些正是麦卢卡、卡努卡和松树精油的关键成分(McDonald et al., 1999; Porter et al., 1998; Porter and Wilkins, 1999)。纳入林牧复合系统的这些树种可通过施氮或截留家畜尿斑,提高精油产量和/或品质,从而创造收益。尿素是否改变植物产品的品质尚需进一步研究。在施氮处理中,麦卢卡和卡努卡在茎生物量中分配的氮均为100 kg N ha−1,而松树仅为35 kg ha−1,所有树种地下部分的氮分配则相近(90–100 kg ha−1)。这些结果表明,就可收获的地上(木材)产品而言,麦卢卡和卡努卡对尿素施肥的响应更好。
At the end of the experiment, a significantly higher total N content was measured in soil after urea application, irrespective of plant species. Similar pH was measured in urea treatments irrespective of plant species; therefore the effect of pH on N loss via NH3 was negligible. At final harvest, pine treatments showed significantly higher moisture contents compared to k�anuka and manuka,� with similar results seen in water filled pore space calculations (Table 1). Analyses of available N showed NO3� as the predominant form, especially in pine and m�anuka treatments, which suggests a high nitrification potential of the soil used in our experiment. The preference of one form of available N over the other can be quite pronounced for a plant species(Britto and Kronzucker, 2013). Britto and Kronzucker (2013) reported that pine seedlings had greater growth and N uptake with NH4+, than NO3�, regardless of pH, temperature or type of growth medium. If pine is less efficient at taking up NO3�, this could explain the higher amount of NO3� in pine treatments in our experiment, compared to only 75 kg ha�1 of NH4+. A rapid conversion of the applied NH4-N into NO3-N hence reduced the preferred N source, and resulted into only low growth response of pine to urea fertilization. Taking into account the low growth response with higher drainage rates in radiata pine, this suggests a potentially higher N loss from pine treatments via leaching, which is confirmed by 53 kg ha�1 NO3-N recovered in pine drainage compared to only 2 kg ha�1 in manuka� and kanuka� (Fig. S2 e supplemental material).
试验结束时,无论何种植物物种,施用尿素后土壤全氮含量均显著较高。尿素处理中各植物物种的pH相近,因此pH对经NH3途径氮损失的影响可忽略不计。最终收获时,松树处理的含水量显著高于卡努卡和麦卢卡,充水孔隙度计算结果与之相似(表1)。有效氮分析表明,NO3−为主要形态,尤其在松树和麦卢卡处理中,这表明本试验所用土壤具有较高的硝化潜力。某一植物物种对某种有效氮形态的偏好可能相当明显(Britto and Kronzucker, 2013)。Britto and Kronzucker(2013)报道,无论pH、温度或生长基质类型如何,松树幼苗在供应NH4+时的生长和氮吸收均优于NO3−。如果松树吸收NO3−的效率较低,则可以解释本试验中松树处理NO3−含量较高,而NH4+仅为75 kg ha−1的现象。施入的NH4-N迅速转化为NO3-N,从而减少了松树偏好的氮源,导致松树对尿素施肥的生长响应较低。考虑到辐射松生长响应较低且排水量较高,这表明松树处理经淋溶途径的氮损失可能更高;松树排水中回收的NO3-N为53 kg ha−1,而麦卢卡和卡努卡仅为2 kg ha−1,证实了这一点(图S2 - 补充材料)。
Kanuka� treatments showed high growth response after urea fertilization with significantly lower NO3-N compared to manuka� and pine, and no significant differences between the two forms NH4-N and NO3-N. This could indicate a non-preferential use of available N sources for plant growth. However, higher amounts of NH4-N in the nitrification assay may also suggest the preference of
卡努卡处理在尿素施肥后表现出较高的生长响应,其NO3-N显著低于麦卢卡和松树,且NH4-N与NO3-N两种形态之间无显著差异。这可能表明其对有效氮源的利用无偏好性。然而,硝化试验中较高的NH4-N含量也可能表明其偏好
NH4-N while at the same time inhibiting nitrification. Since nitrification is a biologically controlled process involving enzymes, mainly ammonia monooxygenase and hydroxylamine oxidoreductase (Robertson and Groffman, 2015), plant species with enzyme inhibiting potential can hence inhibit nitrification (Subbarao et al., 2009). In this context, both, manuka� and k�anuka may inhibit nitrification (Kellam et al., 1992), since results from the nitrification assay showed a slower rate of ammonium reduction in the manuka and k� �anuka treatments compared to pine, resulting in significantly higher NH4-N after 7 and 14 days of assay incubation, respectively. These effects are likely to increase competitiveness of kanuka and m� anuka over other plant species, and therefore explain� and further underline their important role as secondary successional plant species (Franklin et al., 2015; Ross et al., 2009).
NH4-N,同时抑制硝化作用。由于硝化作用是一个由酶参与的生物调控过程,主要涉及氨单加氧酶和羟胺氧化还原酶(Robertson and Groffman, 2015),因此具有酶抑制潜力的植物物种可抑制硝化作用(Subbarao et al., 2009)。在此背景下,麦卢卡和卡努卡均可能抑制硝化作用(Kellam et al., 1992),因为硝化试验结果显示,与松树相比,麦卢卡和卡努卡处理中铵的减少速率较慢,分别在试验培养7天和14天后NH4-N显著较高。这些效应可能增强卡努卡和麦卢卡相对于其他植物物种的竞争力,从而解释并进一步凸显了它们作为次生演替植物物种的重要作用(Franklin et al., 2015; Ross et al., 2009)。
High rates of nitrification lead to high emissions of N2O, especially after rainfall or irrigation (Butterbach-Bahl et al., 2013). This is in accordance with results from our experiments, where a higher N2O flux and higher cumulative N2O emission was detected after urea application in combination with pine, compared to m�anuka and kanuka.� A first peak in N2O emissions between four and six days indicates N2O production during the nitrification process, the conversion from NH4+ to NO3� via NO2�, where NO2� is reduced to N2O (Robertson and Groffman, 2015). Although no differences were detected between tree species at this point, a higher cumulative N2O loss in pine treatments compared to kanuka and m� anuka is in� accordance with results from our nitrification assay, indicating higher nitrification and N2O production during nitrification in soil planted with pine trees. A peak of high N2O emissions was measured 15 days after urea application, most likely because of enzymatic N2O production during denitrification. In contrast, no further increase or N2O peak was detected in kanuka� and m�anuka treatments. This suggests an enzyme inhibiting effect of both, kanuka and m� �anuka during denitrification. Denitrification is driven by individual enzymes, whereas nitrate reductase inhibits the reduction of NO3� to NO2�, the first step in the denitrification pathway (Robertson and Groffman, 2015). In the present study, the N content was determined in several plant parts, soil, leachate and gaseous emissions in form of N2O. Rhizosphere soil was analysed in order to investigate direct effects of different plant species in the same soil type. However, since nitrate and ammonia concentrations in soil vary between rhizosphere and bulk soil (Colin-Belgrand et al., 2003; Zeller et al., 2007), results from this study were not able to provide a complete N mass balance.
高硝化速率会导致较高的N2O排放,尤其是在降雨或灌溉之后(Butterbach-Bahl et al., 2013)。这与本试验结果一致:与麦卢卡和卡努卡相比,松树在施用尿素后检测到更高的N2O通量和更高的累积N2O排放量。第4至6天间出现的第一个N2O排放峰表明N2O产生于硝化过程中,即NH4+经NO2−转化为NO3−的过程,其中NO2−被还原为N2O(Robertson and Groffman, 2015)。尽管此时各树种间未检测到差异,但松树处理的累积N2O损失高于卡努卡和麦卢卡,这与硝化试验结果一致,表明种植松树的土壤中硝化作用及硝化过程中的N2O产生量更高。施用尿素后第15天测得一个高N2O排放峰,很可能是反硝化过程中酶促产生N2O所致。相比之下,卡努卡和麦卢卡处理中未检测到进一步的增加或N2O峰。这表明卡努卡和麦卢卡在反硝化过程中均具有酶抑制效应。反硝化作用由各个酶驱动,其中硝酸还原酶抑制NO3−还原为NO2−,这是反硝化途径的第一步(Robertson and Groffman, 2015)。本研究测定了若干植物部位、土壤、渗滤液以及以N2O形式存在的气态排放中的氮含量。分析根际土壤是为了研究同一土壤类型中不同植物物种的直接效应。然而,由于土壤中硝酸盐和氨的浓度在根际土壤与非根际土壤之间存在差异(Colin-Belgrand et al., 2003; Zeller et al., 2007),本研究结果无法提供完整的氮质量平衡。
5Conclusions结论
Both manuka� and kanuka� responded positively to the addition of urea. Compared to pine, these species had a significant greater positive response. Reduced N leaching and N2O emissions from m�anuka and kanuka compared to pine indicated that these species� may have a similar or better efficacy as pine in reducing nitrification and hence denitrification. These effects could be beneficial in silvopastoral systems, to minimize the amount of N loss via leaching or N2O emissions, by simultaneously increasing plant and stem biomass and potentially increasing and enhancing aboveground plant products. Future research has to verify the benefits of N fertilization on the quality of plant products, and the effect of plant chemicals on microbial communities and enzymes involved in the N cycle. Field studies including these species in combination with different forage crops will verify results in situ and promote alternatives for sustainable silvopastoral systems.
麦卢卡和卡努卡对添加尿素均呈正响应。与松树相比,这些物种的正响应显著更大。与松树相比,麦卢卡和卡努卡的氮淋溶和N2O排放减少,表明这些物种在减少硝化作用进而减少反硝化作用方面可能具有与松树相当或更好的效果。这些效应在林牧复合系统中可能是有益的,可在减少经淋溶或N2O排放途径的氮损失的同时,提高植物和茎干生物量,并有望增加和改善地上植物产品。未来研究需验证施氮对植物产品品质的益处,以及植物化学物质对参与氮循环的微生物群落和酶的影响。将这些物种与不同饲草作物组合的田间研究将在原位验证本研究结果,并推动可持续林牧复合系统替代方案的发展。
Funding基金资助
The study was financially supported by the Deutsche Forschungsgemeinschaft (DFG, ES 416/1-1), the Center of Integrated Biowaste Research (CIBR) as well as Plant & Food Research (Blueskies fund) and Environmental Science and Researach (Pioneer fund).
本研究由Deutsche Forschungsgemeinschaft(DFG, ES 416/1-1)、Center of Integrated Biowaste Research(CIBR)以及Plant & Food Research(Blueskies基金)和Environmental Science and Researach(Pioneer基金)资助。
Acknowledgements致谢
We thank Lowe Environmental Impact for assisting with soil collection, and acknowledge Lincoln University for hosting research. We are grateful to HOV, Q. Liang, Y. Yang, M. Premaratne, T. Parayil-Symon and S. Pokhrel for harvesting assistance and laboratory analyses.
感谢Lowe Environmental Impact协助采集土壤,感谢Lincoln University为本研究提供场所。感谢HOV、Q. Liang、Y. Yang、M. Premaratne、T. Parayil-Symon和S. Pokhrel在收获和实验室分析方面给予的帮助。
Appendix A. Supplementary data附录A. 补充数据
Supplementary data related to this article can be found at http:// dx.doi.org/10.1016/j.envpol.2017.03.042.
本文相关补充数据可见http:// dx.doi.org/10.1016/j.envpol.2017.03.042。
References参考文献
Amaral, J.A., Ekins, A., Richards, S.R., Knowles, R., 1998. Effect of selected monoterpenes on methane oxidation, denitrification, and aerobic metabolism by bacteria in pure culture. Appl. Environ. Microbiol. 64, 520e525.
Beitlich, N., Koelling-Speer, I., Oelschlaegel, S., Speer, K., 2014. Differentiation of manuka honey from kanuka honey and from jelly bush honey using HS-SPME- GC/MS and UHPLC-PDA-MS/MS. J. Agric. Food Chem. 62, 6435e6444.
Bergin, D.O., Kimberley, M.O., Marden, M., 1995. Protective value of regenerating tea tree stands on erosion-prone hill country, East Coast, North Island, New Zealand. N. Z. J. For. Sci. 25, 3e19.
Blakemore, L.C., Searle, P.L., Daly, B.K., 1987. Methods for chemical analysis of soils. N. Z. Soil Bur. Sci. Rep. 80, 9e12.
Britto, D.T., Kronzucker, H.J., 2013. Ecological significance and complexity of Nsource preference in plants. Ann. Bot. 112, 957e963.
Butterbach-Bahl, K., Baggs, E.M., Dannenmann, M., Kiese, R., Zechmeister- Boltenstern, S., 2013. Nitrous oxide emissions from soils: how well do we understand the processes and their controls? Philosophical Trans. R. Soc. B 368, 20130122.
Castaldi, S., Carfora, A., Fiorentino, A., Natale, A., Messere, A., Miglietta, F., otrufo, M.F., 2009. Inhibition of net nitrification activity in a Mediterranean woodland: possible role of chemicals produced by Arbutus unedo. Plant Soil 315, 273e283.
Chang, S.X., Amatya, G., Beare, M.H., Mead, D.J., 2002. Soil properties under a Pinus radiata e ryegrass silvopastoral system in New Zealand. Part I. Soil N and moisture availability, soil C, and tree growth. Agrofor. Syst. 54, 137e147.
Colin-Belgrand, M., Dambrine, E., Bienaime,� S., Nys, C., Turpault, M.-P., 2003. Influence of tree roots on nitrogen mineralization. Scand. J. For. Res. 18, 260e268. Cooper, A.B., 1986. Suppression of nitrate formation within an exotic conifer plantation. Plant Soil 93, 383e394.
Cuttle, S.P., Bourne, P.C., 1993. Uptake and leaching of nitrogen from artificial urine applied to grassland on different dates during the growing season. Plant Soil 150, 77e86.
Eichhorn, M.P., Paris, P., Herzog, F., Incoll, L.D., Liagre, F., Mantzanas, K., Mayus, M., Moreno, G., Papanastasis, V.P., Pilbeam, D.J., Pisanelli, A., Dupraz, C., 2006. Silvoarable systems in europe e past, present and future prospects. Agrofor. Syst. 67, 29e50.
Franklin, H.M., Dickinson, N.M., Esnault, C.J.D., Robinson, B.H., 2015. Native plants and nitrogen in agricultural landscapes of New Zealand. Plant Soil 394, 407e420.
Hawke, M.F., Tombleson, J.D., 1993. Production and interaction of pastures and shelterbelts in the central North Island. In: Proceedings Oftbe NewZealand Grassland Association, pp. 193e197.
Herbert, J.W., Bergin, D.O., Steward, G.A., 1997. Native Trees for Production Forestry. What's New in Forest Research. New Zealand Forest Research Institute Limited. Hutchinson, G.L., Mosier, A.R., 1981. Improved soil cover method for field measurement of nitrous oxide fluxes. Soil Sci. Soc. Am. J. 45, 311e316.
Kellam, S.J., Tisch, M.H., Walker, J.R.L., 1992. Screening of New Zealand native plants for enzyme inhibitory activities. N. Z. J. Bot. 30, 199e203.
Lopez-Díaz, M.L., Rigueiro-Rodríguez, A., Mosquera-Losada, M.R., 2009. In� fluence of
pasture botanical composition and fertilization treatments on tree growth. For. Ecol. Manag. 257, 1363e1372.
Maddocks-Jennings, W., Wilkinson, J.M., Shillington, D., Cavanagh, H., 2005. A fresh look at manuka and kanuka essential oils from New Zealand. Int. J. Aromather. 15, 141e146.
McDonald, G.A., Steward, D., Franich, A.R., 1999. Monoterpene composition of radiata pine (Pinus radiata D.Don) sapwood from a 13 year old progeny trial. Holz als Roh- Werkst. 57, 301e302.
Mohan Kumar, B., Jacob George, S., Jamaludheen, V., Suresh, T.K., 1998. Comparison of biomass production, tree allometry and nutrient use efficiency of multipurpose trees grown in woodlot and silvopastoral experiments in Kerala, India. For. Ecol. Manag. 112, 145e163.
Mosquera-Losada, M.R., Fernandez-Nú� nez, E., Rigueiro-Rodríguez, A., 2006. Pasture,~ tree and soil evolution in silvopastoral systems of Atlantic Europe. For. Ecol. Manag. 232, 135e145.
Mosquera-Losada, M.R., Riguerio, A., McAdam, J., 2005. Silvopastoralism and Sustainable Land Management. CAB International, Wallingford, GB.
Neilsen, W.A., Pataczek, W., Lynch, T., Pyrke, R., 1992. Growth response of Pinus radiata to multiple applications of nitrogen fertilizer and evaluation of the quantity of added nitrogen remaining in the forest system. Plant Soil 144, 207e217.
Northup, R.R., Yu, Z., Dahlgren, R.A., Vogt, K.A., 1995. Polyphenol control of nitrogen release from pine litter. Nature 377, 227e229.
Oenema, O., Velthof, G.L., Yamulki, S., Jarvis, S.C., 1997. Nitrous oxide emissions from grazed grassland. Soil Use Manag. 13, 288e295.
Paavolainen, L., Kitunen, V., Smolander, A., 1998. Inhibition of nitrification in forest soil by monoterpenes. Plant Soil 205, 147e154.
Porter, N.G., Smale, P.E., Nelson, M.A., Hay, A.J., Van Klink, J.W., Dean, C.M., 1998. Variability in essential oil chemistry and plant morphology within a Leptospermum scoparium population. N. Z. J. Bot. 36, 125e133.
Porter, N.G., Wilkins, A.L., 1999. Chemical, physical and antimicrobial properties of essential oils of Leptospermum scoparium and Kunzea ericoides. Phytochemistry 50, 407e415.
Poudel, D.D., Horwath, W.R., Lanini, W.T., Temple, S.R., van Bruggen, A.H.C., 2002. Comparison of soil N availability and leaching potential, crop yields and weeds in organic, low-input and conventional farming systems in northern California. Agriculture, Ecosyst. Environ. 90, 125e137.
Prosser, J., 2011. Manuka (Leptospermum scoparium) as a Remediation Species for Biosolids Amended Land. MSc Thesis. Massey University, New Zealand.
Prosser, J.A., Woods, R.R., Horswell, J., Robinson, B.H., 2016. The potential in-situ antimicrobial ability of Myrtaceae plant species on pathogens in soil. Soil Biol. Biochem. 96, 1e3.
Pyke, N., Chynoweth, R., Mathers, D., 2016. Integrated nutrient and water management for sustainable farming. In: Currie, L.D., Singh, R. (Eds.), The Potential Impact and Opportunities from Nutrient Management Regulation on the New Zealand Herbage Seed Industry. Fertilizer and Lime Research Centre, Massey University, Palmerston North, New Zealand.
Rice, E.L., Pancholy, S.K., 1973. Inhibition of nitrification by climax ecosystems. II. Additional evidence and possible role of tannins. Am. J. Bot. 60, 691e702.
Robertson, G.P., Groffman, P.M., 2015. Nitrogen transformations. In: Paul, E.A. (Ed.), Soil Microbiology, Ecology and Biochemistry. Academic Press, Burlington, Massachusetts, USA, pp. 421e446.
Ross, D.J., Scott, N.A., Lambie, S.M., Trotter, C.M., Rodda, N.J., Townsend, J.A., 2009. Nitrogen and carbon cycling in a New Zealand pumice soil under a manuka (Leptospermum scoparium) and kanuka (Kunzea ericoides) shrubland. Aust. J. Soil Res. 47, 725e736.
Selbie, D.R., Lanigan, G.J., Laughlin, R.J., Di, H.J., Moir, J.L., Cameron, K.C., Clough, T.J., Watson, C.J., Grant, J., Somers, C., Richards, K.G., 2015. Confirmation of codenitrification in grazed grassland. Sci. Rep. 5, 1e9.
Singh, M., Khan, M.M.A., Naeem, M., 2016. Effect of nitrogen on growth, nutrient assimilation, essential oil content, yield and quality attributes in Zingiber officinale Rosc. J. Saudi Soc. Agric. Sci. 15, 171e178.
Song, C.Y., Nam, E.H., Park, S.H., Hwang, C.Y., 2013. In vitro efficacy of the essential oil from Leptospermum scoparium (manuka) on antimicrobial susceptibility and biofilm formation in Staphylococcus pseudintermedius isolates from dogs. Veterinary dermatol. 24, 404e408 e487.
Steinhorn, G., Sims, I.M., Carnachan, S.M., Carr, A.J., Schlothauer, R., 2011. Isolation and characterisation of arabinogalactan-proteins from New Zealand kanuka
honey. Food Chem. 128, 949e956.
Stephens, J.M., Schlothauer, R.C., Morris, B.D., Yang, D., Fearnley, L., Greenwood, D.R., Loomes, K.M., 2010. Phenolic compounds and methylglyoxal in some New Zealand manuka and kanuka honeys. Food Chem. 120, 78e86.
Stephens, J.M.C., Molan, P.C., Clarkson, B.D., 2005. A review of Leptospermum scoparium (Myrtaceae) in New Zealand. N. Z. J. Bot. 43, 431e449.
Subbarao, G.V., Nakahara, K., Hurtado, M.P., Ono, H., Moreta, D.E., Salcedo, A.F., Yoshihashi, A.T., Ishikawa, T., Ishitani, M., Ohnishi-Kameyama, M., Yoshida, M., Rondon, M., Rao, I.M., Lascano, C.E., Berry, W.L., Ito, O., 2009. Evidence for biological nitrification inhibition in Brachiaria pastures. Proc. Natl. Acad. Sci. U. S. A. 106, 17302e17307.
Subbarao, G.V., Sahrawat, K.L., Nakahara, K., Rao, I.M., Ishitani, M., Hash, C.T., Kishii, M., Bonnett, D.G., Berry, W.L., Lata, J.C., 2013. A paradigm shift towards low-nitrifying production systems: the role of biological nitrification inhibition (BNI). Ann. Bot. 112 (2), 297e316. http://dx.doi.org/10.1093/aob/mcs230. https://www.ncbi.nlm.nih.gov/pubmed/23118123.
Suescun, F., Paulino, L., Zagal, E., Ovalle, C., Munoz, C.,~ 2012. Plant extracts from the Mediterranean zone of Chile potentially affect soil microbial activity related to N transformations: a laboratory experiment. Acta Agriculturae Scandinavica. Sect. B d Soil & Plant Sci. 62, 556e564.
Tsamaidi, D., Karapanos, I.C., Passam, H.C., Daferera, D., Polissiou, M., 2012. The Yield and Composition of Dill Essential Oil in Relation to N Application, Season of Cultivation and Stage of Harvest. International Society for Horticultural Science (ISHS), Leuven, Belgium, pp. 189e194.
White, C.S., 1988. Nitrification inhibition by monoterpenoids: theoretical mode of action based on molecular structures. Ecology 69, 1631e1633.
Wyatt, R.M., Hodges, L.D., Kalafatis, N., Wright, P.F., Wynne, P.M., Macrides, T.A., 2005. Phytochemical analysis and biological screening of leaf and twig extracts from Kunzea ericoides. Phytotherapy Res. PTR 19, 963e970.
Zeller, B., Recous, S., Kunze, M., Moukoumi, J., Colin-Belgrand, M., Bienaime,� S., Ranger, J., Dambrine, E., 2007. Influence of tree species on gross and net N transformations in forest soils. Ann. For. Sci. 64, 151e158.